Dr. Avinash Gholave
Department of Botany
K.V. N. Naik Arts, Commerce And Science College Nashik.
agholave@gmail.com
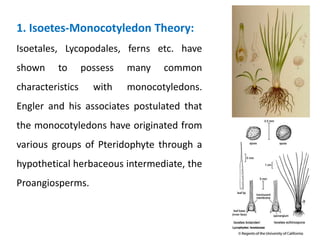
1. Isoetes-Monocotyledon Theory:
Isoetales, Lycopodales, ferns etc. have
shown to possess many common
characteristics with monocotyledons.
Engler and his associates postulated that
the monocotyledons have originated from
various groups of Pteridophyte through a
hypothetical herbaceous intermediate, the
Proangiosperms.
According to Campbell (1928) the
herbaceous angiosperms are primitive,
those inherited from filicinean ancestor.
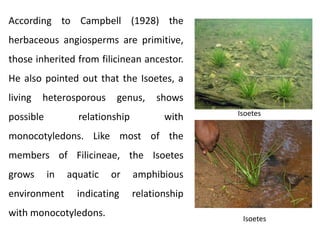
He also pointed out that the Isoetes, a
living heterosporous genus, shows
possible relationship with
monocotyledons. Like most of the
members of Filicineae, the Isoetes
grows in aquatic or amphibious
environment indicating relationship
with monocotyledons.
Isoetes
Isoetes
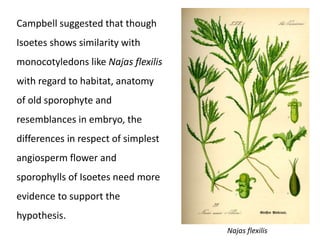
Campbell suggested that though
Isoetes shows similarity with
monocotyledons like Najas flexilis
with regard to habitat, anatomy
of old sporophyte and
resemblances in embryo, the
differences in respect of simplest
angiosperm flower and
sporophylls of Isoetes need more
evidence to support the
hypothesis.
Najas flexilis
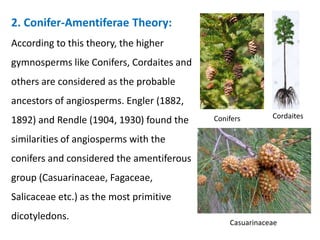
The Lycopodiales and Equisetales
are now considered as completely
separate and independent
evolutionary lines.
The monocots are now
considered to be more advanced
than dicotyledons and their
resemblance with Isoetes is
superficial in nature.
Lycopodiales
Equisetales
2. Conifer-Amentiferae Theory:
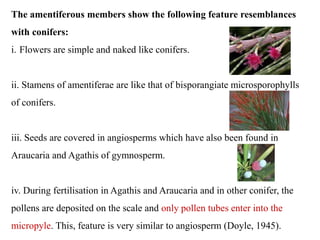
According to this theory, the higher
gymnosperms like Conifers, Cordaites and
others are considered as the probable
ancestors of angiosperms. Engler (1882,
1892) and Rendle (1904, 1930) found the
similarities of angiosperms with the
conifers and considered the amentiferous
group (Casuarinaceae, Fagaceae,
Salicaceae etc.) as the most primitive
dicotyledons.
Conifers Cordaites
Casuarinaceae
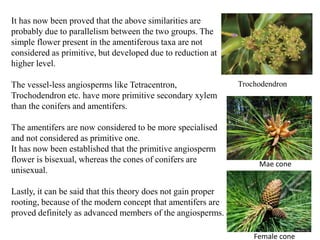
The amentiferous members show the following feature resemblances
with conifers:
i. Flowers are simple and naked like conifers.
ii. Stamens of amentiferae are like that of bisporangiate microsporophylls
of conifers.
iii. Seeds are covered in angiosperms which have also been found in
Araucaria and Agathis of gymnosperm.
iv. During fertilisation in Agathis and Araucaria and in other conifer, the
pollens are deposited on the scale and only pollen tubes enter into the
micropyle. This, feature is very similar to angiosperm (Doyle, 1945).
It has now been proved that the above similarities are
probably due to parallelism between the two groups. The
simple flower present in the amentiferous taxa are not
considered as primitive, but developed due to reduction at
higher level.
The vessel-less angiosperms like Tetracentron,
Trochodendron etc. have more primitive secondary xylem
than the conifers and amentifers.
The amentifers are now considered to be more specialised
and not considered as primitive one.
It has now been established that the primitive angiosperm
flower is bisexual, whereas the cones of conifers are
unisexual.
Lastly, it can be said that this theory does not gain proper
rooting, because of the modern concept that amentifers are
proved definitely as advanced members of the angiosperms.
Trochodendron
Mae cone
Female cone
3. Gnetales-Angiosperm Theory:
Richard von Wettstein (1901) emphasised the
close relationship between Gnetales and
angiosperms, after modifying the Engler’s system
as mentioned in Handbuch der Systematische
Botanik.
Later on, Markgraf (1930) and Fagerlind (1947)
boldly supported the above view. Fagerlind
demonstrated the homology among the three
genera of Gnetales (Ephedra, Welwitschia and
Gnetum) and proposed that Gnetales and Pro-
angiosperms evolved from a common ancestor.
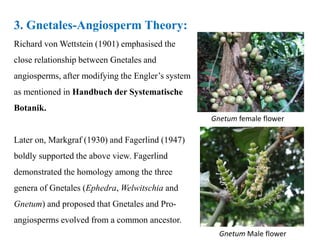
Gnetum female flower
Gnetum Male flower
Similarities between Gnetales and Angiosperms:
i. Presence of two cotyledons. ii. Vessels in the secondary wood.
iii. Venation – reticulate.
iv. Unisexual inflorescence (similar to catkin of many Amentifers).
Gnetum wood cross section
Gnetum leaf
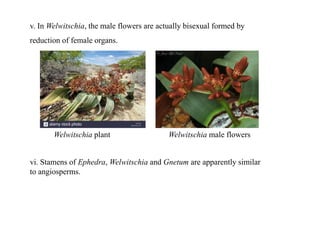
v. In Welwitschia, the male flowers are actually bisexual formed by
reduction of female organs.
vi. Stamens of Ephedra, Welwitschia and Gnetum are apparently similar
to angiosperms.
Welwitschia plant Welwitschia male flowers
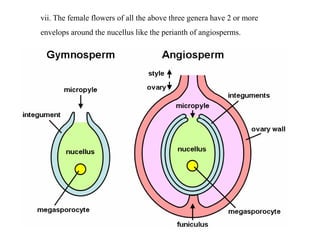
vii. The female flowers of all the above three genera have 2 or more
envelops around the nucellus like the perianth of angiosperms.
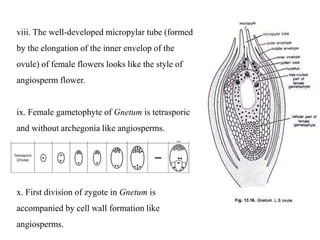
viii. The well-developed micropylar tube (formed
by the elongation of the inner envelop of the
ovule) of female flowers looks like the style of
angiosperm flower.
ix. Female gametophyte of Gnetum is tetrasporic
and without archegonia like angiosperms.
x. First division of zygote in Gnetum is
accompanied by cell wall formation like
angiosperms.
Differences between Gnetales and Angiosperms:
i. Gnetum have vessels in secondary wood, while it is absent in some
primitive dicots like Tetracentron, Trochodendron, etc.
ii. The vessels of Gnetales originate in an entirely different way from those
of angiosperms.
iii. The presence of scalariform pitted tracheids, a characteristic of primitive
angiosperms, is absent in both primary and secondary xylem of Gnetum.
While circular bordered pits appear in Gnetum during the ontogeny of
secondary xylem.
iv. Gnetum also differs from angiosperms in respect of development of
vessels.
Based on the above discussions, it can be said that the similarity between
Gnetales and certain angiosperms is now considered as superficial and
appears due to tilting towards convergence during evolution. Similarities
in the number of cotyledons (two) also appear due to convergence.
The angiosperms might have been evolved from polycotyledonous
ancestors rather than dicotyledonous one. The polycotyledon (3-4
cotyledones) is reported in an extant genus Degeneria, a primitive group
of angiosperm. The absence of archegonia in Gnetum indicates its
affinity with angiosperms due to parallelism. But the vascular anatomy
strongly opposes any suggestion regarding the relationship between
angiosperms and Gnetales.
4. Bennettitalean Theory:
According to Saporta and Marion
(1885), and Arber and Parkin
(1907), the Bennettitales of
gymnosperm is the possible
ancestor of angiosperms. They
considered Benettitales as the
possible ancestor of angiosperms
due to similarities between the
strobili of Cycadeoidea, a Mesozoic
genus and the flower of Magnolia.
Similarities:
i. Both the structures (strobili and flower)
are bisexual having an elongated central
axis.
ii. In Cycadeoidea the different parts like
bracts, microsporophylls and
megasporophylls are arranged from the
bottom towards the apex, while in
Magnolia, perianth, stamens and carpels
are arranged in a similar way.
In spite of the above superficial similarities,
both the groups show much differences by
the detail investigation.
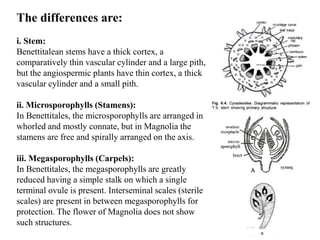
The differences are:
i. Stem:
Benettitalean stems have a thick cortex, a
comparatively thin vascular cylinder and a large pith,
but the angiospermic plants have thin cortex, a thick
vascular cylinder and a small pith.
ii. Microsporophylls (Stamens):
In Benettitales, the microsporophylls are arranged in
whorled and mostly connate, but in Magnolia the
stamens are free and spirally arranged on the axis.
iii. Megasporophylls (Carpels):
In Benettitales, the megasporophylls are greatly
reduced having a simple stalk on which a single
terminal ovule is present. Interseminal scales (sterile
scales) are present in between megasporophylls for
protection. The flower of Magnolia does not show
such structures.
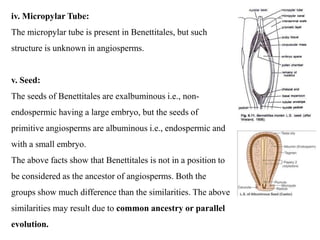
iv. Micropylar Tube:
The micropylar tube is present in Benettitales, but such
structure is unknown in angiosperms.
v. Seed:
The seeds of Benettitales are exalbuminous i.e., non-
endospermic having a large embryo, but the seeds of
primitive angiosperms are albuminous i.e., endospermic and
with a small embryo.
The above facts show that Benettitales is not in a position to
be considered as the ancestor of angiosperms. Both the
groups show much difference than the similarities. The above
similarities may result due to common ancestry or parallel
evolution.
According to Arber and Parkin (1907), both the groups have a
common origin from seed ferns and they might have diversed
very early. Later, Takhtajan (1980) mentioned in his
classification that Magnoliophyta are regarded to be
monophyletic in origin, most probably derived from
Bennettitale-like ancestors or stocks ancestral to them.
Armen Takhtajan
5. Pteridosperm Theory:
The Pteridosperms are also known as Cycadofilicales or
seed ferns. They are so called because the plants show
fernlike leaves; some of them bears leaves associated with
cycadlike stem showing difference in stem anatomy with
ferns. They bear true seeds.
They were reported abundantly from Upper Devonian to
Permian of Paleozoic Age. Plants are often monoecious,
but micro- and megasporophylls are not arranged in
definite strobili. Based on the above characteristics of
stem, leaf and seed, they are considered as the probable
ancestors of Bennettitales. Cycadofilicales
The various evidences and interpretations discussed the
possibility of Cycadales, Bennettitales or any other
gymnosperms to be the ancestor of angiosperms. Therefore,
emphasis was given to the Pteridosperms as the possible
ancestor. Cronquist (1968) stated that “it is a long way,
morphologically, from any known seed fern to an
angiosperm, but each of the differences could logically be
bridged in the course of evolution”.
The angiosperms show double fertilisation with triploid (3n)
endosperm, possibly due to reduction of female
gametophyte. Likewise, sepals originate from leaves and
petals from both sepals and stamens.
Thus the evolution of an angiospermic flower
can be traced from cones or cone-like structures
of gymnosperms. Further more, the primitive
angiosperm like Magnolia lacks vessels in
secondary woods is similar to seed ferns. Thus,
angiosperms could have evolved from a
Pteridospermous ancestry.
Melville (1960) stated that the reproductive
branch of Glossopteridales (Pteridosperm) is
somewhat comparable with the present-day
angiosperm Dichapetalum.
Glossopteridales
Dichapetalum
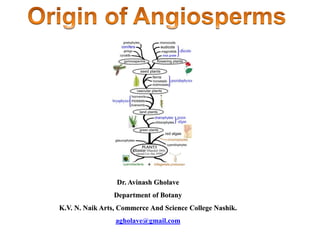
Origin of Angiosperm