An Overview ofPlant
Development (Part II)
Post-embryonic Phase
[From Developmental Biology, Eighth Edition,
by Scott F. Gilbert, published by Sinauer Associates, Inc.]
Susan R. Singer
Laurence McKinley Gould Professor of the Natural Sciences,
Carleton College
Reporter: Kimberly Rose P. Balmeo
2.
An Overview ofPlant
Development (Part II)
Germination
Vegetative Growth
The Vegetative-to-Reproductive
Transition
Senescence
3.
Germination
the resumptionof the growth of the seed
embryo after the period of dormancy
In order to takes place
A period of After-ripening
Seed-Environment Interaction
Stratification (requirement of chilling)
Imbibition (rehydration)
Scarification (scratched or etched)
4.
Germination
During germination
Gibberellins trigger the breakdown of
starch into sugar.
Light trigger differentiation of chloroplast
Radicle
5.
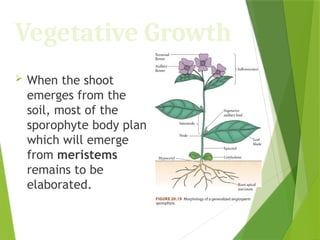
Vegetative Growth
Whenthe shoot
emerges from the
soil, most of the
sporophyte body plan
which will emerge
from meristems
remains to be
elaborated.
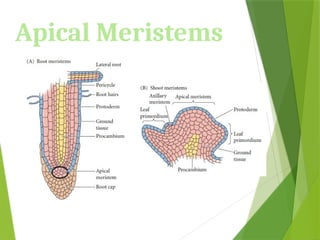
Apical Meristems
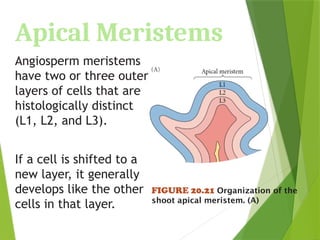
Angiosperm meristems
havetwo or three outer
layers of cells that are
histologically distinct
(L1, L2, and L3).
If a cell is shifted to a
new layer, it generally
develops like the other
cells in that layer.
FIGURE 20.21 Organization of the
shoot apical meristem. (A)
9.
Apical Meristems
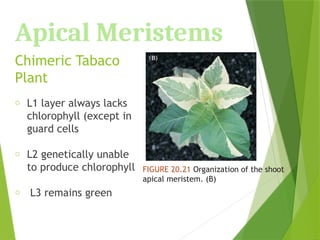
Chimeric Tabaco
Plant
oL1 layer always lacks
chlorophyll (except in
guard cells
o L2 genetically unable
to produce chlorophyll
o L3 remains green
FIGURE 20.21 Organization of the shoot
apical meristem. (B)
10.
Apical Meristems
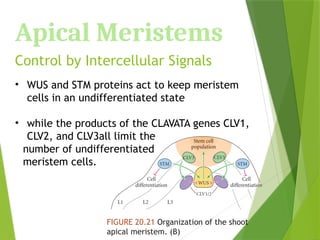
Control byIntercellular Signals
• WUS and STM proteins act to keep meristem
cells in an undifferentiated state
• while the products of the CLAVATA genes CLV1,
CLV2, and CLV3all limit the
number of undifferentiated
meristem cells.
FIGURE 20.21 Organization of the shoot
apical meristem. (B)
11.
Meristems
Apical Meristem
Shoot
Root
Lateral Meristem – secondary growth
Intercalary Meristem – inserted in the
stems of monocot between mature tissues
12.
Root Development
Radialand axial patterning – from
embryogenesis throughout development
as the primary root grows and lateral
roots emerge from pericycle
13.
Root Development
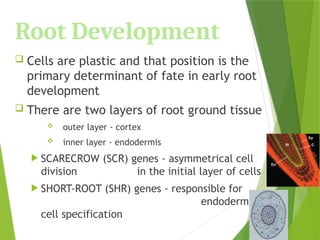
Cellsare plastic and that position is the
primary determinant of fate in early root
development
There are two layers of root ground tissue
outer layer - cortex
inner layer - endodermis
SCARECROW (SCR) genes - asymmetrical cell
division in the initial layer of cells
SHORT-ROOT (SHR) genes - responsible for
endodermal
cell specification
14.
Root Development
Distributionof the plant hormone auxin
organizes the axial pattern.
A peak in auxin concentration at the root
tip must be perceived for normal axial
patterning
15.
Shoot Development
ApicalDominance
Branching patterns are
regulated by the shoot
tip
Plant Hormones
Auxin - suppresses the
outgrowth of axillary bud
Cytokinin - release buds
from apical dominance
Axillary buds can initiate
their own axillary buds
environmental
signals
maximizes light
capture
Asymmetrical tree
crowns form when
two trees grow very
close to each other
shoot architecture
is genetically
regulated
16.
Shoot Development
Phyllotaxy- involves communication
among existing and newly forming leaf
primordial
the mature sporophyte is created by stacking
node/internode units together
mechanisms for maintaining geometrically
regular spacing of leaves on a plant
17.
Shoot Development
cells’commitment to become a leaf
research indicates that the youngest visible
leaf primordia are not determined to make a
leaf; rather, programming for leaf
development occurs only later
establishment of the leaf axes
morphogenesis
Leaf Shape
Apoptosis
Differential cell growth
18.
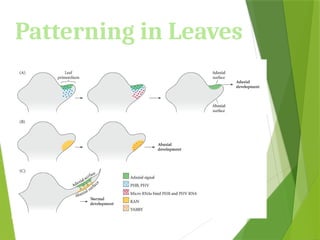
Patterning in Leaves
DORSAL-VENTRAL / adaxial side-abaxial side
PHABUL OSA (PHB) and PHAVOLUTA (PHV) genes
initially have uniformly expressed RNA throughout the
primordium
proteins are receptors for an adaxial signal, which
leads to the accumulation of PHB and PHV on the
adaxial leaf surface
KANADI (KAN) genes initiate abaxial cell differentiation
Abaxial fate also appears to be specified by three
members of the YABBY gene family
Patterning in Leaves
SIMPLE AND COMPOUND LEAVES
Whether simple and compound leaves develop by the same mechanism is
an open question
Class I KNOX genes are homeobox genes that include STM and the
KNOTTED 1 (KN1) gene in maize – mutation causes meristem-like
bumps to form on maize leaves
When KN1, or the tomato homologue LeT6, with a promoter from
cauliflower mosaic virus, the gene is expressed at high levels
throughout the plant, and the leaves become "super compound"
In response to overexpression of KN1 Simple leaves become more
lobed (but not compound),
consistent with the hypothesis that compound leaves may be an
extreme case of lobing in simple leaves
consistent with the hypothesis that compound leaves are
modified shoots.
21.
Patterning in Leaves
SIMPLE AND COMPOUND LEAVES
Whether simple and compound leaves develop by the same
mechanism is an open question
Class I KNOX genes are homeobox genes that include STM
and the KNOTTED 1 (KN1) gene in maize – mutation causes
meristem-like bumps to form on maize leaves
In wild-type plants KNOX genes stimulate meristem
initiation and growth
YABBY genes (some) - function by downregulating KNOX
genes - Control KN1 gene
22.
Patterning in Leaves
SIMPLE AND COMPOUND LEAVES
Whether simple and compound leaves develop by the same
mechanism is an open question
When KN1, or the tomato homologue LeT6, with a promoter
from cauliflower mosaic virus, the gene is expressed at high
levels throughout the plant, and the leaves become "super
compound"
In response to overexpression of KN1 Simple leaves become
more lobed (but not compound),
hypotheses
compound leaves may be an extreme case of lobing in simple
leaves
compound leaves are modified shoots
23.
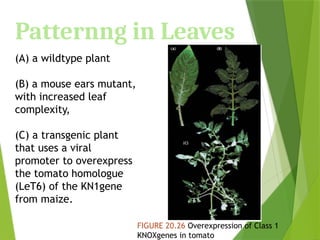
Patternng in Leaves
(A)a wildtype plant
(B) a mouse ears mutant,
with increased leaf
complexity,
(C) a transgenic plant
that uses a viral
promoter to overexpress
the tomato homologue
(LeT6) of the KN1gene
from maize.
FIGURE 20.26 Overexpression of Class 1
KNOXgenes in tomato
24.
Patternng in Leaves
(A)Wild-type pea plant
(B) The tl mutant, in
which tendrils are
converted to leaflets
(C) The af mutant, in
which leaflets are
converted to tendrils
(D) An af tl double
mutant, which results in a
“parsley leaf” phenotype
FIGURE 20.28 Leaf morphology mutants in
peas
25.
Vegetative-to-Reproductive
Transition
vegetative andreproductive structures of the
shoot are all derived from the shoot meristem
formed during embryogenesis
Maximal reproductive success in angiosperms
depends on the timing of flowering and on
balancing the number of seeds produced with
the resources allocated to individual seeds
a signal from the leaves moves to the shoot
apex and induces flowering
26.
Vegetative-to-Reproductive
Transition
Signals toflowering
environmental conditions
Photoperiodism
Chronological age of the plant
Size of plant
Temperature
The nature of the flowering signal,
however, remains unknown.
27.
Vegetative-to-Reproductive
Transition
JUVENILITY
juvenilephase - the plant cannot produce
reproductive structures even if all the
appropriate environmental signals are present
EARLY PHASE CHANGE (EPC) gene in maize is
required to maintain the juvenile state
Arabidopsis juvenility gene HASTY (HST),
necessary for microRNA processing and export
from the nucleus. Loss of-function mutants
undergo early phase change because microRNAs
are trapped in the nucleus
28.
Vegetative-to-Reproductive
Transition
FLORAL SIGNALS
The “black box” between environmental signals
and the production of a flower is vanishing
rapidly
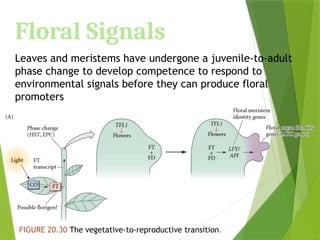
CONSTANS (CO) responds to day length,
promoting flowering under long-day conditions,
activates transcription of a gene called
FLOWERING LOCUS T (FT).
FT is transcribed only in the leaves, but the
transcript travels through the phloem (transport
tissue) from the leaf to the shoot and is likely
translated when it arrives at the shoot meristem
29.
Floral Signals
Leaves andmeristems have undergone a juvenile-to-adult
phase change to develop competence to respond to
environmental signals before they can produce floral
promoters
FIGURE 20.30 The vegetative-to-reproductive transition.
30.
Senescence
developmental programleading to death,
is closely linked to flowering in many
angiosperms
Fruit ripening (and ultimately overripening) is an
example of organ senescence
Monocarpic plants flower once and then senesce.
Polycarpic plants, such as the bristlecone pine, can
live thousands of years (4,900 years is the current
record) and flower repeatedly.
Editor's Notes
#3 Dormancy - not actively growing:, in order to survive adverse environmental conditions
Stratification – Chilling, optimum temperature, drying/desiccation
#13 clonal analyses and laser ablation experiments